Easter, 2026
On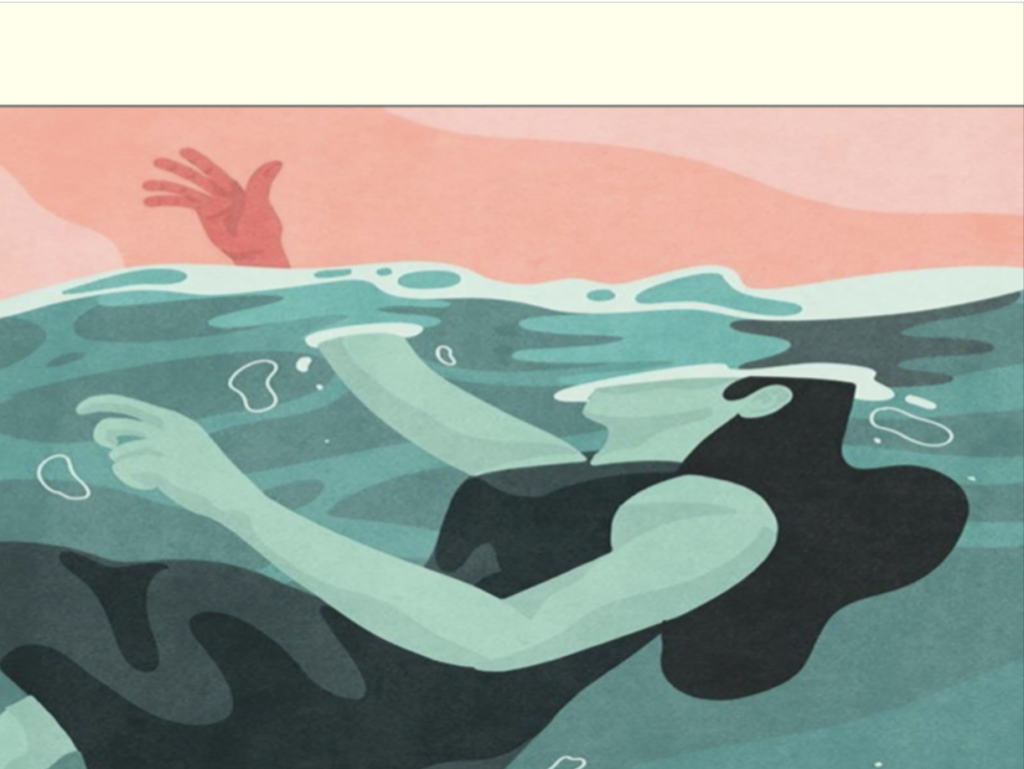
The hardcover edition of W.B. Yeats’ A Terrible Beauty Is Born, published by Grapevine India, does not credit the cover illustrator as Indian publishing houses typically use anonymous in-house graphic designers. They should have made an exception for this one, an image which mingles the possibilities of birth and death to provide a haunting counter-point to Yeats’ wonderful poem about the uncertainty of certainty.
Yeats’ leitmotif, which should be part of any honest scientist’s stock in trade, runs through my own life and work as far back as I can remember. Today, I will try to apply that duality to the newly born star, Cardiovascular-Kidney-Metabolic (CKM) Syndrome.
A 2026 Boston-based study uncovered CKM in 80% of young socioeconomically deprived North Americans (1). 800 of a thousand men and women with a mean age of 23 were found to be flotsam in the toxic metabolic inner sea created by today’s food industry, and drifting towards their first heart attack or stroke. Not all of them will reach those end-points; CKM also increases the risk of liver failure, kidney failure, multi-organ damage and premature death from all causes.
But CKM is not really new. It is a formal medical framework which derives from the earlier concept of metabolic ill health, and extends and quantifies it. Stage 1, for example, is characterized by abdominal adiposity and prediabetes; Stage 2 incorporates Type 2 diabetes, high blood pressure, high triglycerides or moderate chronic kidney disease (CKD); Stage 3 contains pre-clinical cardiovascular disease such as arterial re-modelling, and Stage 4 includes major cardiovascular events (MACE).
None of the Boston findings were really new either.
In 2019 a University of North Carolina study had found that 88% of all Americans were metabolically unhealthy (2), and in 2022 a Tufts University study generated a similar figure (3), with an estimated 40% of all Americans estimated to be at the equivalent of CKM Stages 2 and 3.
The subjects in the 2026 study, however, were young Americans. The finding that 20-year-olds were almost as susceptible to metabolic ageing as the average American – median age 39.4 (4) – was shocking and, for many, counter-intuitive.
Why is this happening? Equally importantly, can this trend be stopped before the storm surge of newly diseased young and middle-aged men and women swamps what is left of our healthcare systems? Drugs cannot be the answer. Only the most ideologically rigid doctors can still cleave to the pharmaceutical model when dealing with problems so obviously derived from our lifestyle.
Pharmaconutritional programs offer an alternative that is inarguably safer, and arguably more effective. Arguable, because the trials needed to prove them cannot be done unless governments start to show a real interest in the health of their constituents; a phenomenon which has not been seen on any scale since the 60’s, when Sir Richard Peto’s work ultimately enabled mandatory health warnings for tobacco products and Ralph Nader drove car safety technology deep into Detroit.
If you ask what drives CKM, the answer you generally get is hyper-nutrition. Excess calories and obesity lead to metabolic dysregulation, and thence to CKM. But there are several steps along the way, and each step is potentially a metabolic and nutritional nexus where pharmaconutritional modifiers can be introduced to prevent the decline into CKM.
Three of the steps are the Endoplasmic Reticular Stress response, the Integrated Stress Response and the Cell Danger Response, which form three nested and progressive tiers of buffering. (nb CDR is not as well documented as the first two, and may be an extension of ISR).
The entry-level buffer is endoplasmic reticular stress (ERS). Protein folding, which takes place in the endoplasmic reticulum, is a complex procedure with a high failure rate; only 20% of proteins are configured correctly, and if this low figure drops the integrity of the cell becomes compromised. Chronic hyperglycemia (6) and hyperlipidemia (7) both disrupt the endoreticular environment, driving up levels of malfolded proteins which trigger ERS.
ERS unleashes the Unfolded Protein Response, in which increased production of chaperones (8) attempts to restore correct folding to acceptable levels. If the cause is time-restricted, such as a week of ultra-processed foods with a high content of sugars and lipids (pick your poison), an acute ERS / UPR ensues. This entirely adaptive process restores normality.
Longer-term consumption of modern ultra-processed foods works differently. As with inflammation, where acute is usually productive and chronic is overwhelmingly destructive, chronic ERS induced by bad dietary habits is harmful. Much of the harm is mediated via the mitochondria, which are close-coupled to the endoplasmic reticulum at mitochondria-associated ER membranes aka MAMs.
Chronic endoplasmic reticulum stress causes mitochondrial malfunction via calcium overload (9). This impairs the electron transport chain, causing a drop in ATP production and a surge in mitochondrial Reactive Oxygen Species (mtROS). And this triggers the Integrated Stress Response (10).
The Integrated Stress Response (ISR) is the second tier of buffering, and its function is to preserve not just the ER but the whole cell.
Here again, an acute ISR is adaptive; it turns down protein synthesis, sparing the cell’s energy and slowing the build-up of malfolded proteins which might otherwise damage or kill the cell. It maintains production of only those proteins essential for cellular survival, clears out cellular damage, triggers mitochondrial biogenesis in order to regenerate sufficient energy for the damaged cell and buys the cell time to recover from environmental shocks such as nutrient deprivation or viral infection (11).
If the cause of the ISR is sustained, however, for example via chronic ERS and in any situation where the original stressor cannot be resolved, the ISR is re-programmed. It becomes the chronic Integrated Stress Response program (12, 13), promotes further mitochondrial dysfunction and sustained oxidative stress and enters a ‘Janus’ pathway. The ISR has given up on trying to save the affected cell and has now switched to killing it; a strategic retreat designed to protect surrounding tissue by eliminating an irreparably damaged (ie virally infected or cancerous) cell.
If the ISR is chronically activated it graduates to the Cell Danger Response, which may simply be chronic ISR acting on a larger scale ie in larger areas of tissue (14). The CDR is thought to progress through three stages. If all goes well then Phase 1 can be categorized as up-regulated defense and containment, Phase 2 is repair and Phase 3 is restoration and re-connection.
Under persistent ISR stress, damaged and dying cells leak ATP into the extracellular space. Extracellular ATP is a biochemical alarm that has been postulated to alert neighboring cells and, when present in excess, trap them in a chronic CDR loop leaving the affected tissues in CDR-1 (15). This terrible and beautiful theory was proposed by Dr Robert Naviaux at UCSD (14).
According to this theory sustained oxidative stress, lipid peroxidation and chronic inflammation then drive progressive tissue damage, via progressive degradation of the extracellular matrix. At this point CDR becomes clinically important, or at least symptomatic, and the degenerative condition driven by CDR-1 will worsen over time.
The oft-cited trio of omega 3 PUFAs, polyphenols and prebiotic fibers comes in here.
Omega-3s damp ERS and therefore the ISR via multiple mechanisms (16, 17). They also damp the CDR by suppressing pro-inflammatory pathways (18), stimulating the antioxidant regulator NRF2 (19) and by producing Specialized Pro-Resolving Mediators (SPMs) resolvins and protectins which instruct immune and injured cells to stop the cell danger response (20).
Polyphenols (various) damp ERS & ISR via reducing protein malfolding. They are reported to up-regulate cellular production of endogenous chaperones (21), to act on occasion as chaperones themselves (22) and to reduce ROS in the endoplasmic reticulum (23) and associated mitochondria (24, 25).
The prebiotic fibers work in parallel. They damp ERS & thus the ISR via microbial production of short chain fatty acids, especially butyrate (26). Fascinatingly, in light of butyrate’s known ability to kill a range of cancer cells (ie 27), it increases ERS in cancer cells and induces the Chronic Integrative Stress program (28) which leads to cell death.
The prebiotics also switch off the ISR and CDR via two additional and entirely different routes. In the first and more established of these, the prebiotic-induced shift in colonic microbiota and the resulting reduction in colonic epithelial inflammatory stress switches off the ISR-inducing enzyme indoleamine oxidase 1 (29-31).
When indoleamine oxidase 1 (IDO1) is activated by chronic inflammation, this causes a fall in levels of its substrate l-tryptophan. Falling tryptophan levels mimic starvation, a stressor which activates the ISR (32). To make matters worse, IDO1 metabolizes tryptophan to kynurenine, a mitochondrial toxin (33) which makes ISR worse.
This is not a good idea if your ISR is already over-activated, which it probably is. The same junk food diet that causes dysbiosis and creates chronic inflammatory stress in the large bowel and activates IDO1, is simultaneously driving chronic ERS and ISR via hyperglycemia and hyperlipidemia.
Prebiotics induce eubiosis and reduce colonic inflammation (31), thus damping inflammation-driven IDO1 (32). Less IDO1 activity means increased tryptophan and decreased kynurenine, both of which down-regulate the ISR (33, 34) – but there is more. When IDO1 is switched off, tryptophan metabolism shifts from the kynurenine pathway to the indole and indole-3-acetic acid (3-IAA) pathway (35), which inter alia produces indole propionic acid (IPA).
The switch from kynurenine to 3-IAA is associated with multiple health benefits (ie (36, 37). It cannot be coincidental that 3-IAA and IPA are mito-protective (38, 39) and down-regulate the ISR (340).
New evidence suggests a second prebiotic protective mechanism. Some probiotic species produce exopolysaccharides which induce mitochondrial biogenesis (41), which would improve cellular energy production and thus damp both ERS and ISR.
All of this appears highly relevant to public health. Intakes of omega 3 PUFAs, polyphenols and prebiotic fibers have fallen precipitously in the shift from unprocessed to increasingly ultraprocessed diets; and they have been replaced by sugars and fats.
The growing global tides of non-communicable degenerative disease have been linked by multiple authors to the declining quality of the modern food table, in which traditional nutrient density has been displaced by calorific density. Logically, restoring a traditional dietary profile would reverse most of the adverse health trends that have increasingly disfigured public health over the last 3 or 4 generations, and provide us with the relative freedom from degenerative disease enjoyed by the Mid-Victorians (42), and the latter-day Hadzabe (43) and Tsimane (44).
In this post I have tried to lay out a set of less familiar mechanisms whereby a small number of pharmaconutritional tools switch off the damaging chronic inflammation that is at the core of so much chronic degenerative disease. They re-set our fevered and pro-inflammatory milieu interieur into a new (but really traditional) anti-inflammatory configuration in which healing can predominate, and chronic degenerative disease pushed back.
The machinery is increasingly well documented, the numbers of cases I and my colleagues see expand continuously, and my certainty of the validity of this approach grows. But I am uncertain, and will remain so until these theories, and the burgeoning number of successful case histories, can be put to the sword of the randomised and prospective clinical trial.
Until that happens many millions of Pearces, Connollys, Guptas, Zhangs and Schmidts will sicken and die prematurely, metaphorically executed by a firing squad of multinational food and pharmaceutical companies, together with their political enablers.
What I am certain of is that this must change – but when? A terrible beauty, a beauty which will radically re-shape the corporate world and in the process make us all healthier and happier, is still waiting to be born.
References:
- Krishnan V, Ning H, Notterman DA, Goldman N, Khan SS, Shah NS, Allen NB, Lloyd-Jones DM. Association Between Cardiovascular-Kidney-Metabolic Health and Early Arterial Injury in Young Adults in the United States: The Future of Families-Cardiovascular Health Among Young Adults Study. Circ Popul Health Outcomes. 2026 Aug 20:e013042.
- Araújo J, Cai J, Stevens J. Prevalence of Optimal Metabolic Health in American Adults: National Health and Nutrition Examination Survey 2009-2016. Metab Syndr Relat Disord. 2019 Feb;17(1):46-52.
- O’Hearn M, Lauren BN, Wong JB, Kim DD, Mozaffarian D. Trends and Disparities in Cardiometabolic Health Among U.S. Adults, 1999-2018. J Am Coll Cardiol. 2022 Jul 12;80(2):138-151.
- https://www.census.gov/library/stories/2026/04/age-and-sex.html
- https://drpaulclayton.eu/blog/disorderly-conduct/
- Morales-Rivera MI, Martínez-Portilla RJ, Orozco L. Relevant Serum Endoplasmic Reticulum Stress Biomarkers in Type 2 Diabetes and Its Complications: A Systematic Review and Meta-Analysis. Antioxidants (Basel). 2024 Dec 19;13(12):1564.
- Sozen E, Ozer NK. Impact of high cholesterol and endoplasmic reticulum stress on metabolic diseases: An updated mini-review. Redox Biol. 2017 Aug;12:456-461.
- Ni M, Lee AS. ER chaperones in mammalian development and human diseases. FEBS Lett. 2007 Jul 31;581(19):3641-51.
- Mohsin AA, Thompson J, Hu Y, Hollander J, Lesnefsky EJ, Chen Q. Endoplasmic reticulum stress-induced complex I defect: Central role of calcium overload. Arch Biochem Biophys. 2020 Apr 15;683:108299.
- Mick E, Titov DV, Skinner OS, Sharma R, Jourdain AA, Mootha VK. Distinct mitochondrial defects trigger the integrated stress response depending on the metabolic state of the cell. Elife. 2020 May 28;9:e49178.
- Costa-Mattioli M, Walter P. The integrated stress response: From mechanism to disease. Science. 2020 Apr 24;368(6489):eaat5314.
- Guan BJ, van Hoef V, Jobava R, Elroy-Stein O, Valasek LS, Cargnello M, Gao XH, Krokowski D, Merrick WC, Kimball SR, Komar AA, Koromilas AE, Wynshaw-Boris A, Topisirovic I, Larsson O, Hatzoglou M. A Unique ISR Program Determines Cellular Responses to Chronic Stress. Mol Cell. 2017 Dec 7;68(5):885-900.e6.
- Altintas DM, Cerqua M, Comoglio PM, Chaveroux C. The Janus framework of the integrated stress response: from homeostasis to maladaptation. Life Sci Alliance. 2025 Dec 29;9(3):e202503523.
- Naviaux RK. Metabolic features of the cell danger response. Mitochondrion. 2014 May;16:7-17. doi: 10.1016/j.mito.2013.08.006. Epub 2013 Aug 24.
- Trautmann A. “Extracellular ATP in the immune system: more than just a ‘danger signal’.” Science Signaling, 2009;2(56):pe6.
- Sullivan EM, Pennington ER, Green WD, Beck MA, Brown DA, Shaikh SR. Mechanisms by Which Dietary Fatty Acids Regulate Mitochondrial Structure-Function in Health and Disease. Adv Nutr. 2018 May 1;9(3):247-262.
- Warda F, Graham L, Batch-Joudi J, Gupta N, Mooradian AG. Omega-3 Fatty Acids Inhibit Endoplasmic Reticulum (ER) Stress in Human Coronary Artery Endothelial Cells. J Food Biochem (2023), https://doi.org/10.1155/2023/7300030
- Kar A, Ghosh P, Patra P, Chini DS, Nath AK, Saha JK, Pagtra BC. Omega-3 fatty acids mediated Cellular signaling and its regulation in Human Health. (2023). Clin Nut Open Sci 52, 72-86
- Quarta S, Santarpino G, Calabriso N, Carluccio MA, Siracusa L, Strano T, Cardetta F, Siculella L, Damiano F, De Caterina R, Massaro M. Omega-3 PUFAs reduce inflammation by targeting NRF2 and NF-κB activity in an ex vivo model of cardiac mature adipocytes and adipose derived stem cells from atherosclerotic patients. Food Funct. 2026 Feb 9;17(3):1431-1450.
- Poggioli R, Hirani K, Jogani VG, Ricordi C. Modulation of inflammation and immunity by Omega-3 fatty acids: a possible role for prevention and to halt disease progression in autoimmune, viral, and age-related disorders. Eur Rev Med Pharm Sci (2023). 27: 7380-7400
- Hajieva P. The Effect of Polyphenols on Protein Degradation Pathways: Implications for Neuroprotection. Molecules. 2017 Jan 19;22(1):159.
- Leri M, Scuto M, Ontario ML, Calabrese V, Calabrese EJ, Bucciantini M, Stefani M. Healthy Effects of Plant Polyphenols: Molecular Mechanisms. Int J Mol Sci. 2020 Feb 13;21(4):1250.
- Raffiei H, Omidian K, Bandy B. Protection by different classes of dietary polyphenols against palmitic acid-induced steatosis, nitro-oxidative stress and endoplasmic reticulum stress in HepG2 hepatocytes. J Funct Foods (2018). 44, 173-182
- Ashkar F, Bhullar KS, Wu J. The Effect of Polyphenols on Kidney Disease: Targeting Mitochondria. Nutrients. 2022 Jul 29;14(15):3115.
- Maksimović T, Gădău C, Antal G, Čoban M, Eșanu O, Atyim E, Mioc A, Șoica C. Polyphenol-Based Therapeutic Strategies for Mitochondrial Dysfunction in Aging. Biomolecules. 2025 Aug 3;15(8):1116.
- Kushwaha V, Rai P, Varshney S, Gupta S, Khandelwal N, Kumar D, Nilkanth Gaikwad A. Sodium butyrate reduces endoplasmic reticulum stress by modulating CHOP and empowers favorable anti-inflammatory adipose tissue immune-metabolism in HFD fed mice model of obesity. Food Chem (Oxf). 2022 Jan 25;4:100079.
- Wang W, Fang D, Zhang H, Xue J, Wangchuk D, Du J, Jiang L. Sodium Butyrate Selectively Kills Cancer Cells and Inhibits Migration in Colorectal Cancer by Targeting Thioredoxin-1. Onco Targets Ther. 2020 May 27;13:4691-4704.
- Zhang J, Yi M, Zha L, Chen S, Li Z, Li C, Gong M, Deng H, Chu X, Chen J, Zhang Z, Mao L, Sun S. Sodium Butyrate Induces Endoplasmic Reticulum Stress and Autophagy in Colorectal Cells: Implications for Apoptosis. PLoS One. 2016 Jan 19;11(1):e0147218.
- Ciorba MA. Indoleamine 2,3 dioxygenase in intestinal disease. Curr Opin Gastroenterol. 2013 Mar;29(2):146-52.
- Salminen A. Role of indoleamine 2,3-dioxygenase 1 (IDO1) and kynurenine pathway in the regulation of the aging process. Ageing Res Rev. 2022 Mar;75:101573.
- Roy S, Dhaneshwar S. Role of prebiotics, probiotics, and synbiotics in management of inflammatory bowel disease: Current perspectives. World J Gastroenterol. 2023 Apr 14;29(14):2078-2100.
- Martin-Gallausiaux C, Larraufie P, Jarry A, Béguet-Crespel F, Marinelli L, Ledue F, Reimann F, Blottière HM, Lapaque N. Butyrate Produced by Commensal Bacteria Down-Regulates Indolamine 2,3-Dioxygenase 1 (IDO-1) Expression via a Dual Mechanism in Human Intestinal Epithelial Cells. Front Immunol. 2018 Dec 11;9:2838.
- Metz R, Rust S, Duhadaway JB, Mautino MR, Munn DH, Vahanian NN, Link CJ, Prendergast GC. IDO inhibits a tryptophan sufficiency signal that stimulates mTOR: A novel IDO effector pathway targeted by D-1-methyl-tryptophan. Oncoimmunology. 2012 Dec 1;1(9):1460-1468.
- Nagy-Grócz G, Spekker E, Vécsei L. Kynurenines, Neuronal Excitotoxicity, and Mitochondrial Oxidative Stress: Role of the Intestinal Flora. Int J Mol Sci. 2024 Jan 30;25(3):1698.
- Hou Y, Li J, Ying S. Tryptophan Metabolism and Gut Microbiota: A Novel Regulatory Axis Integrating the Microbiome, Immunity, and Cancer. Metabolites. 2023 Nov 20;13(11):1166.
- Shi C, Dong J, Hui X, Xu Z, Zhao Z, Dong L. Production, Mechanisms, and Therapeutic Strategies of Tryptophan Metabolites in CNS Diseases. Mol Neurobiol. 2025 Dec 1;63(1):226.
- Lu Z, Zhang C, Zhang J, Su W, Wang G, Wang Z. The Kynurenine Pathway and Indole Pathway in Tryptophan Metabolism Influence Tumor Progression. Cancer Med. 2025 Mar;14(6):e70703.
- Zhang C, Fu Q, Shao K, Liu L, Ma X, Zhang F, Zhang X, Meng L, Yan C, Zhao X. Indole-3-acetic acid improves the hepatic mitochondrial respiration defects by PGC1a up-regulation. Cell Signal. 2022 Nov;99:110442.
- Li Q, de Oliveira Formiga R, Puchois V, Creusot L, Ahmad AH, Amouyal S, Campos-Ribeiro MA, Zhao Y, Harris DMM, Lasserre F, Ellero-Simatos S, Guillou H, Huang Z, Brot L, Hu Y, Chollet L, Danne C, Scandola C, Ledent T, Chevreux G, Argüello RJ, De Carvalho Bittencourt M, Bettinger J, D’Aveni-Piney M, Moulin D, Schreiber S, Aden K, Rolhion N, Michel ML, Wai T, Sokol H. Microbial metabolite indole-3-propionic acid drives mitochondrial respiration in CD4+ T cells to confer protection against intestinal inflammation. Nat Metab. 2025 Dec;7(12):2510-2530.
- Yu X, Li W, Feng H, Li Z, Zheng H, Sun S, Li J, Li B, Wu Q. A Mediterranean-mimicking diet harnesses gut microbiota–derived 3- IAA to rejuvenate T cell. eLIFE Reviewed Preprint v1 • February 12, 2026
- Prajapati SK, Yadav D, Katiyar S, Jain S, Yadav H. Postbiotics as Mitochondrial Modulators in Inflammatory Bowel Disease: Mechanistic Insights and Therapeutic Potential. Biomolecules. 2025 Jul 1;15(7):954.
- Clayton P, Rowbotham J. How the mid-Victorians worked, ate and died. Int J Environ Res Public Health. 2009 Mar;6(3):1235-53.
- Sayre MK, Anyawire M, Paolo B, Mabulla AZP, Pontzer H, Wood BM, Raichlen DA. Lifestyle and patterns of physical activity in Hadza foragers. Am J Biol Anthropol. 2023 Nov;182(3):340-356.
- Gurven M, Kaplan H, Trumble B, Stieglitz J. The Biodemography of Human Health in Contemporary Non-industrial Populations: Insights from the Tsimane Health and Life History Project. https://gurven.anth.ucsb.edu/sites/default/files/sitefiles/papers/gurvenetalHEDbookchapter.pdf